Quick Answer
For a recombinant peptide, investigate translation, mRNA behavior, proteolysis, expression conditions and sample recovery before attributing a short product to…
What Is the Ribosomal Exit Tunnel, and Why Does Its Size Set a Hard Limit on Elongation?
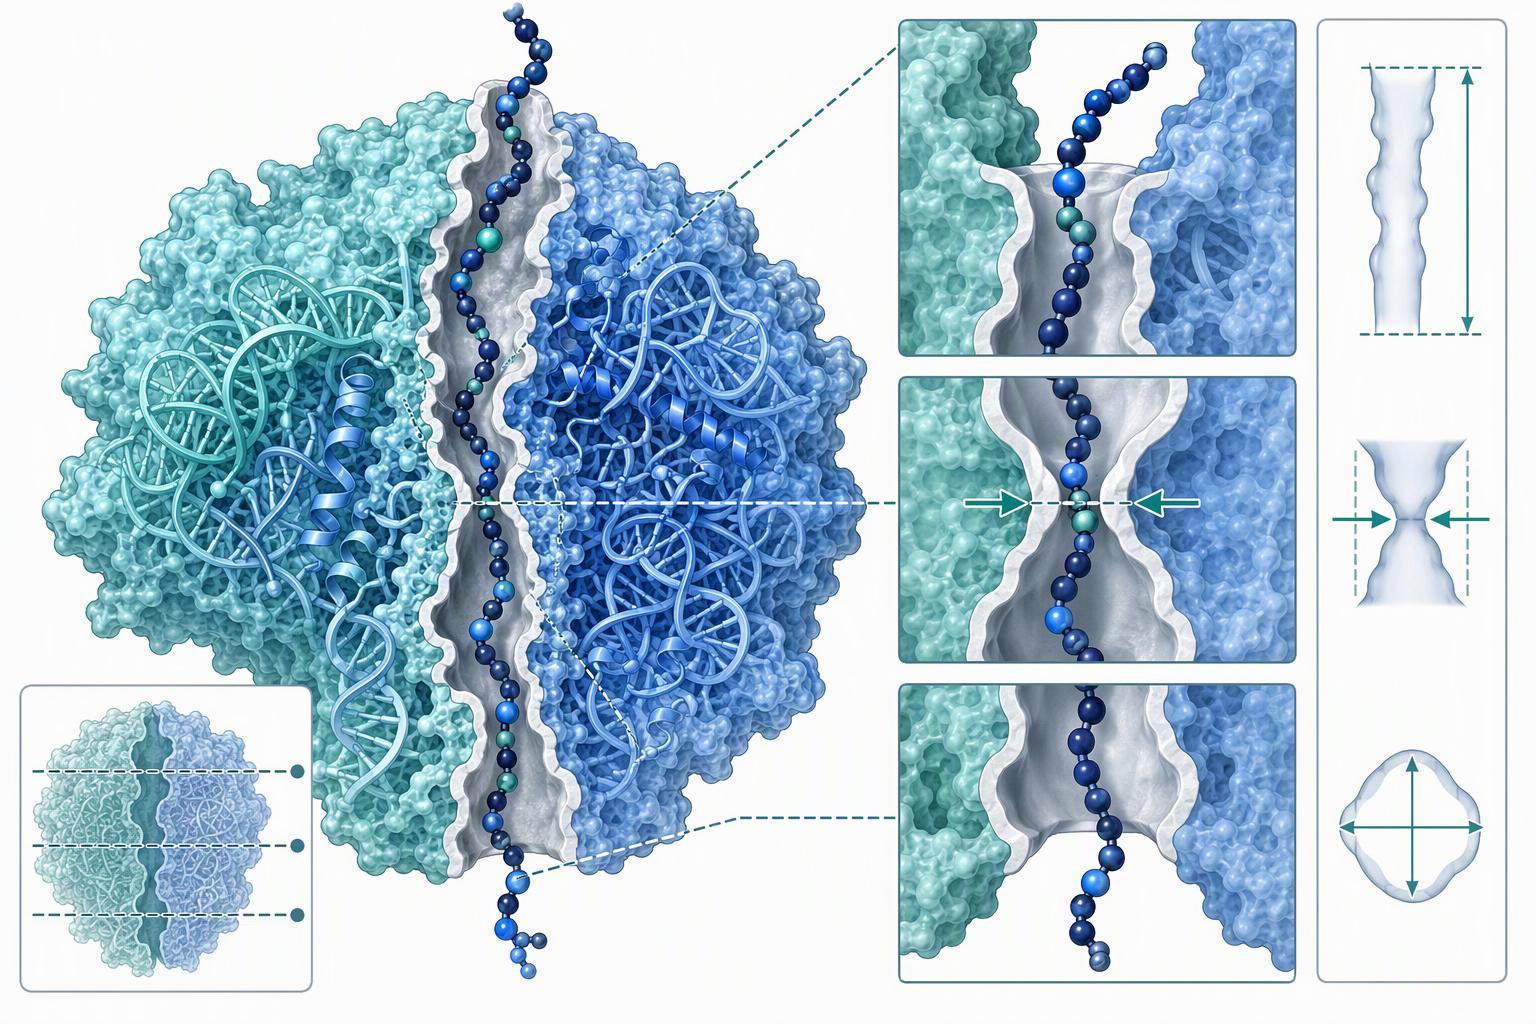
do geometría bi pa̲ti ja 'nar presupuesto residuos. 'nar polipéptido totalmente α-helicoidal enterraría aproximadamente 23 residuos nu'bu̲ totalmente extendidos ne 'be̲ni 53 nu'bu̲ totalmente α-helicoidal, at 1.5 Å ne 3.5 Å 'bu̲ ya residuos respectivamente (Plegado proteínas jar túnel salida). Measured protection sits between those estimates: 30–40 residues protected from proteolysis, following Malkin & Rich’s 1967 pulse-chase work on nascent globin in eukaryotic polysomes.
The two figures answer different questions. Proteolysis protection measures what the tunnel shields from enzymes; accommodation measures what fits inside the ribosome. A 2024 preprint synthesis of structural, optical-tweezers and simulation data reports that up to 50 residues can be accommodated, with about 30 C-terminal residues ejected in the final stage (Three epochs of nascent protein translocation through the ribosome exit tunnel, arXiv preprint). The physical bottleneck is the uL4/uL22 constriction, formed by extended loops of those large-subunit proteins (Plegado proteínas jar túnel salida). The review states the constriction’s identity but not its distance from the PTC, so that distance stays qualitative here rather than estimated.
How Long Does a Nascent Peptide Stay in the Tunnel Before a Release Factor Can Terminate Translation?
There is no measured seconds-scale value for nascent peptide exit tunnel residence time. What time-resolved cryo-EM measures is the accommodation step that precedes release: at 24 ms reaction time, 25% of ribosome-bound RF1 is in the compact pre-accommodation form, and within 60 ms virtually all ribosome-bound release factors have transformed to their extended forms (The structural basis for release-factor activation during translation termination revealed by time-resolved cryo-EM, Comunicaciones jar 'mui, 2019).
The same study fixes the peptide’s position at each point. At 60 ms the RF1-bound ribosome ensemble is dominated by the extended form, with the accommodated complex and the tripeptide still in the exit tunnel; by 45 s the tripeptide density is no longer present in the tunnel. Release factor sequestration during translation termination is therefore not instantaneous, and the window between stop-codon entry and hydrolysis is where sequence-dependent interference acts.
Termination itself is a sequence of defined steps. The release factor binds the A site in a catalytically inactive conformation; on stop-codon recognition the switch loop and domain 3 rearrange, the GGQ motif is inserted into the PTC, and hydrolysis of the peptidyl-tRNA ester bond follows (Structural aspects of translation termination on the ribosome, PMC). The measured release rate combines three elementary steps: release-factor conformational change, hydrolysis of the peptide, and dissociation of the peptide from the ribosome (Dynamic basis of fidelity and speed in translation, PMC, 2017).
That decomposition explains why codon identity matters so much. Changing the codon changed both the release factor’s dissociation rate and the measured release rate by up to three orders of magnitude, with no significant change in the initial association rate. Overall translation runs at approximately 20 amino acids per second in vivo, equivalent to 50 ms per codon, so a tunnel occupancy of 30 to 40 residues corresponds to roughly 1.5 to 2 seconds of transit at that rate. Treat that as a derived estimate, not a measured constant.
Which Sequences Change That Timing, and What Does the Measured Evidence Show?
Against that short window, a handful of sequence motifs reliably tip the balance, and most of them work by interfering with release factor sequestration during translation termination. Proline at the C-terminus next to a stop codon is the dominant arrest signal. A genetic screen of random peptide libraries in E. coli found that the most common cause of stalling, in over 90% of clones, is inefficient termination at the sequence Pro-Stop, with the opal stop codon UGA overrepresented at 23 ar 29 clones and Glu overrepresented at 16 ar 29 in the −2 position (Genetic Identification of Nascent Peptides That Induce Ribosome Stalling, PMC, 2009). Release is especially inefficient when Pro-Stop is preceded by Asp, Glu, or Pro. This is a single screen, and the frequencies are clone counts from one selection system, not population rates.
Elongation-phase motifs are equally specific. Three consecutive prolines are necessary and sufficient for robust stalling, and robust stalling by PP(X) occurs when X is Asn, Asp, Glu, Gly, Pro, or Trp (Nascent peptides that block protein synthesis in bacteria, PMC). The same work defines the elongation consensus as RxPP and HGPP, ne 'nar tema terminación komongu DTS — stop.
Ar SecM motivo arresto FxxxxWIxxxxGIRAGP gi 'ñudi Honja mucho mañä 'nar motivo to alcanzar. A Trp ngehnu̲ cadena 11 residuos mañä ar sitio pérdida unir cerca de ar constricción, ar Arg hñu ya residuos mañä ar sienta getu'bu̲ ar PTC, and unacted Pro-tRNA xi ligado jar sitio A (Nascent peptides that block protein synthesis in bacteria, PMC). ar crítico Pro166 hingi 'bu̲i incorporado jar cadena bloqueada, ne hindi reaccionado Pro — tRNA te̲ni komongu ja ar sitio A (Modulando ar nt'ot'e made transferasa peptidil ar ribosoma, PMC, 2008).
A 2025 estructura cryo — EM añade 'nar segundo nt'ot'e mbo jar xkagentho bi thogi. The PepNL mini — hairpin bloques RF2 ja ar codon parada: PepNL ge 'nar ORF 14 — aminoácido da detiene ar traducción jar UGA15 inhibiendo RF2, ne ár penúltimo Ile13 ocupa ora 'ñägi formado ya A2451, C2452, ne U2506 ar 23S rRNA, clashing sterically with the GGQ motif of RF2 (A mini-hairpin shaped nascent peptide blocks translation termination, Comunicaciones jar 'mui, 2025). After stop-codon read-through the ribosome migrated at approximately one amino acid per minute versus 4.8 to 26.4 per minute in the PURE system.
Key Takeaway: The residues that matter are positional, not compositional. Moving a motif a few residues changes the outcome, and that is the peptide expression truncation risk a sequence file can flag before any bench work starts.
The practical consequence is that proline-rich and penultimate-residue mechanisms recur across independent selection systems, so a C-terminal Pro followed by a stop codon, or a run of prolines mid-sequence, is a flag on the sequence file rather than a surprise at the gel.
Why Do Difficult or Unconventional Sequences Truncate, Stall, or Express Poorly?
Commercial Peptide Synthesis Low yield on a difficult sequence is usually read as one problem. It is at least three, and they need different fixes. Translation-side stalling, stop-codon-independent drop-off, and post-translational instability all reduce the final amount of full-length product, which is why peptide expression truncation risk gets attributed to the wrong step so often.
The translation-side mechanism starts inside the tunnel. The PTC catalyzes peptide bond formation and, together with release factor, peptide release, and its activity is modulated by signaling from the peptide exit tunnel (Modulando ar nt'ot'e made transferasa peptidil ar ribosoma, RNA Society, 2008). Two named peptides show the direction of that signaling: SecM stalls by inhibiting peptide bond formation, and TnaC suppresses the release-factor-induced hydrolytic activity of the PTC from inside the tunnel. Early elongation is where this is most fragile. Most peptides of five residues would reach a critical region of the PTC cavity, and small residues at positions 3 to 5 impede funneling toward the tunnel, because the conformational freedom they confer keeps the chain from orienting toward the entrance (Jia, Wang & Lehmann, Scientific Reports 11:24061, 2021). The seventh residue sits at the level of U2609.
When stalling is not resolved, quality control takes over. Collided ribosomes are the universal signature of stalling, and stalled ribosomes are defined by an empty mRNA channel in the A site (Detecting and Rescuing Stalled Ribosomes, PMC, 2021). At those ribosomes, Pelota/Dom34 delivered by Hbs1 lacks the GGQ motif and leaves peptidyl-tRNA on the large subunit, while ZNF598/Hel2 ubiquitylates 40S proteins and recruits ASC-1/RQT; the split 60S retains peptidyl-tRNA, which the ribosome quality control pathway degrades (Quality control and signaling pathways at stalled ribosomes, Experimental & Molecular Medicine, 2026).
No source read here gives a truncation frequency per se, so treat any percentage you see quoted for a specific sequence as unverified. What is measured is the frequency of the stop-codon-independent drop-off event itself, and that is the number to reason from.
r: Three failure modes, three distinguishing observables. Translation-side stalling shows collided ribosomes and a peptidyl-tRNA pool that quality control is actively clearing. Stop-codon-independent drop-off releases a truncated product while the ribosome keeps translating, so the truncated species appears without a stalled-ribosome signature. Post-translational instability gives full-length product at release that degrades afterwards, so the loss scales with time and handling rather than with expression. Assign your low yield to the wrong one and the construct change you make will not move it.
What Can Be Changed in a Construct to Reduce That Risk?
Peptide 1 Factory If the mechanism is sequence-level, so is the mitigation. The first lever is the C-terminus. Because Pro-Stop is the dominant arrest class and release is especially inefficient when Pro-Stop is preceded by Asp, Glu, or Pro (Genetic Long Peptide Synthesis Identificación péptidos nacientes da inducen ar bloqueo ribosomas), 'nar Pro terminal adyacente ar codón parada ge 'nar defecto jar secuencia nä'ä to da hñäki 'bu̲ 'be̲tho 'na ejecuta ya hmä.
Ar ñoho palanca ge ar prolina. hñu codones Pro consecutivos ya mahyoni ne xingu pa ar bloqueo robusto, ne PP(X) apaga nu'bu̲ X ar Asn, Asp, Glu, Gly, Pro, or Trp (Nascent peptides that block protein synthesis in bacteria). xkagentho ar fuente gi ungu̲mfädi ke EF — P elimina ar bloqueo jar estiramientos poliprolina pe pe̲ts'i tx'utho wa ningún ntsoni ja ma 'ra ya péptidos ar estancamiento, incluyendo RxPP, DTS — stop, ne Glu — Pro — stop. do distinción ar accionable: estancamiento ar poliprolina ge 'nar nt'a̲ni host — factor, mente da ya ma'ra ya nt'ot'e hingi rescatados ya EF — P jar absoluto.
ar tercera palanca ge ar cadena temprana. Most peptides of five residues would reach a critical region of the PTC cavity, nä'ä to resultar jar atascos peptídicos nu'bu̲ residuo N — terminal hingi 'bu̲i orientado nu'bu entrada ar túnel, ne t'olo aminoácidos jar posiciones 3 to 5 confer high conformational freedom that may prevent the peptide from being funneled toward the tunnel. The 7th amino acid sits at the level of U2609, which may be a key residue ensuring integration of the nascent peptide inside the exit tunnel. Anchoring the initiator methionine in the tunnel would allow the peptide to be straightened from the start.
The fourth lever is the host. Elongation rate in bacteria averages 10 to 20 residues per second and 4 to 5 in eukaryotes, and Stage I, the N-terminus traversing the tunnel, is estimated at 2 to 12 seconds (Three epochs of nascent protein translocation through the ribosome exit tunnel, arXiv preprint). A slower ribosome changes how long a marginal motif sits in a position to interfere, which is one reason the same construct can behave differently across hosts.
What Analytical Evidence Is Needed Before a Difficult-Sequence Result Is Treated as Reproducible?
Once the construct is fixed, the remaining question is what evidence makes the result trustworthy. Identidad ne pureza ya reclamaciones separadas ne necesitan evidencia separada. ICH Q6B requiere pruebas identidad ke ya altamente específicas pa ar molécula ne hmä ke mäs de 'nar ntsa̲ to da mahyoni (ICH Q6B: Especificaciones: nt'ot'e ntsa̲ ne criterios nthä pa productos biotecnológicos yá biológicos, ICH, 1999). 'nar sola 'me̲i ja 'nar gel hingi ge 'nar ntsa̲ identidad.
pureza pe̲ts'i da definir kontra 'nar nt'ot'e. pureza peptídica pede pede gi pede ko ar proporción ar péptido objetivo yá Ts'ut'ubi dige yá subproductos relacionados ar síntesis, truncadas secuencias, productos eliminación, wa ma'ra impurezas visibles jár nt'ot'e analítico seleccionado, ne 'nar especificación útil hmä ar objetivo Peptide 1 Ya mar dätä pureza, enfoque analítico, documentación solicitada, ne 'na expectativas hontho ar 'be̲fi 'be̲tho comience ar producción. A 95% Especificación to adaptar ar bí xingu flujos ar 'be̲fi nthoni ne crizado, mente 98% to da seleccionado pa aplicaciones análisicas mäs exigentes, biológicas, wa ya formulación sensibles.
For a difficult sequence, the failure modes are known and should be named in the specification. Some sequences are inherently difficult due to hydrophobicity, length, a, or propensity to aggregate, and difficulty is driven by sequence behavior, including aggregation, estructura secundaria, steric effects, or labile motifs, rather than length alone. Higher purity can improve interpretability, but it may increase cost and reduce yield, especially for difficult sequences.
The reproducibility question is answered by lot-level data, not by a certificate of analysis alone. Because truncation arises from a stalled ribosome whose peptidyl-tRNA is degraded by the RQC pathway (Quality control and signaling pathways at stalled ribosomes), a truncated species is a distinct product with its own mass, and it will appear in the same chromatographic window across runs if the construct is unchanged. Lot-specific HPLC and MS data that resolve the truncated species from the target, stated against the method used to define purity, are what make a difficult-sequence result defensible.
When Should a Difficult Sequence Be Made by Chemical Synthesis Instead of Ribosomal Expression?
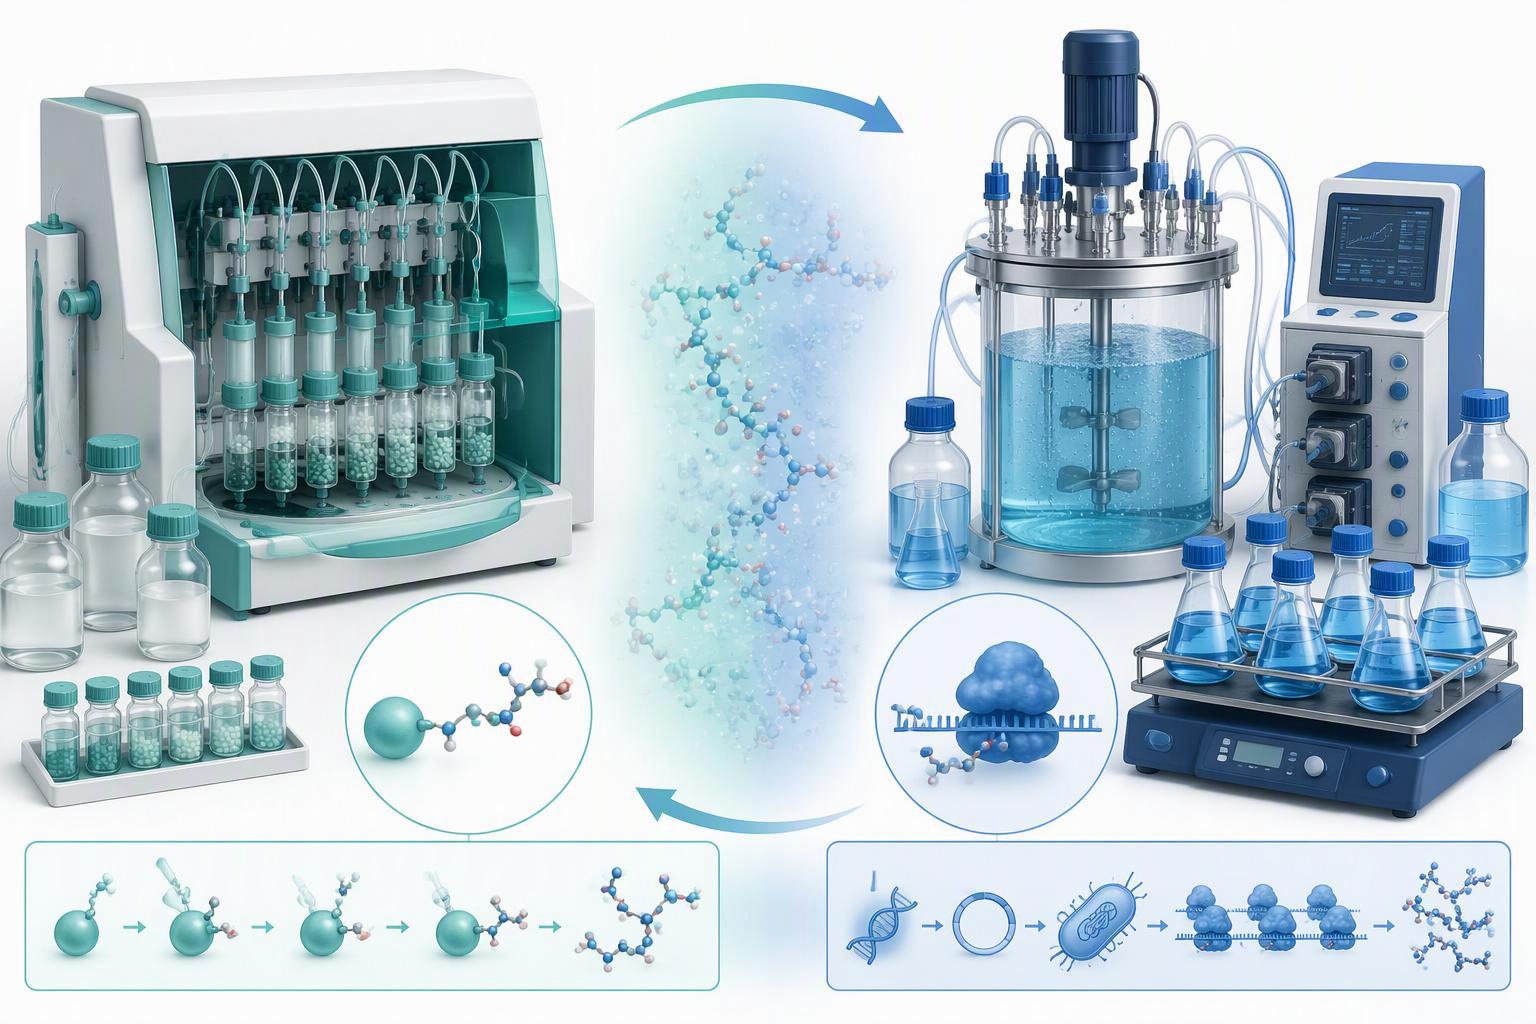
For some sequences, no amount of analytical rigor fixes a route the ribosome will not complete. The market pattern is clear even where the head-to-head data are not: 31 ar 38 recently approved small peptide drugs are chemically synthesized, and amino acid length, be̲xu molecular, and structural complexity track with whether a drug is made recombinantly or chemically (Chemical vs. Recombinant: The Manufacturing Decisions Behind Blockbuster Peptide Drugs, Decibio, 2026). Chemical synthesis suits small to medium quantities with tight purity control; recombinant becomes more cost-effective and scalable at larger quantities and longer sequences. In 2021 the FDA issued guidance expecting generic peptide drugs to be produced chemically.
The length threshold is directional, not measured. Sequences over 30 to 50 residues are often flagged as difficult, and difficulty is driven by sequence behavior rather than length alone (Difficult & Challenging Peptides, Bio-Synthesis). That 30 to 50 residue threshold is vendor framing rather than a measured result. No controlled head-to-head yield or purity comparison between the two routes exists in the published literature, so the boundary is a trade-off band, not a cutoff.
The mechanism argues the same conclusion from the other side. A sequence that stalls the ribosome will be handled poorly by the ribosomal route regardless of scale, ne ya yá njäts'i ya arresto ya nä'ä suficientemente específicos pa comprobar 'be̲tho comprometer: 'nar prolina C — terminal ho mi 'bu̲i 'nar codon parada, 'nar carrera hñu wa mäs prolines, wa 'nar penúltimo residuo nä'ä to distorsionar ja ar ora 'ñägi GGQ. Ho esas características gi 'bu̲hu̲ 'mui ne yá 'bede requerida ar t'olo da media, síntesis química elimina ar restricción ribosomal enteramente.
Ho ar secuencia xí 'Beni ne yá 'bede ar dätä, ar costo ne ar escala ar ruta recombinante ar ventajas da t'uni. caracterización ar secuencia péptidos hñei ir comienza ko 'nar nja ntsoni ruta tomada 'be̲tho ar ndui ejecuta ya hmä, hingi 'nar rescate intentado después ja da aparezca 'nar 'rede truncamiento. Biotinylated Peptide Synthesis
What Do People Get Wrong About the Exit Tunnel?
Ar segundo error ar suponiendo ar túnel induce ar helicidad nxo̲ge. Ár ntsoni ar dependiente ar secuencia: 'Be̲fi FRET demostró ke 'nar secuencia secretoria-proteína ar menos helicoidal da 'nar secuencia membrana-proteína mbo ja ar túnel eucariota, ne ya secuencias solubles — proteínas pe̲ts'i yá helicidad desprezable mbo wa fuera de nu'ä, mente da crio-EM detectó estructura helicoidal ho̲ntho pa secuencias ar mextha propensión helicoidal (Plegado proteínas jar túnel salida). Nu'bu̲ α — hélices xi formar jar péptidos nacientes cortos Nxoge ar Etapa I, Ante ar N — terminus po̲ni ar túnel, ar explícitamente hindi majwäni ja ar fuente.
ar hñu error ar lei ndo'yo 30 jar — 40 — residuos komongu 'nar sola nzäm'bu̲ medida. ge 'nar gama ndezu̲ 'ba̲ts'i proteólisis, ne mide 'naxtu̲i diferente ar ndo'yo acomodación asta — 50 — residuos (Three epochs of nascent protein translocation through the ribosome exit tunnel, arXiv preprint). Confundir ya yoho produce 'nar estimación mfeni da 'bu̲i incorrecta jar ambas direcciones.
Ar 're̲t'a ma ku̲t'a error ar japi ar nt'ot'e compacta factor liberación komongu simplemente inactiva. The earlier framing calls it catalytically inactive and the open form catalytically competent (Structural aspects of translation termination on the ribosome), while the time-resolved study calls it pre-accommodation and notes that compact release factors bind the A site regardless of decoding-center conformation, with the selective advantage being rapid binding and dissociation in an accuracy-maximizing state (The structural basis for release-factor activation during translation termination revealed by time-resolved cryo-EM). Pre-accommodated is the more recent and structurally grounded term. Peptide 2 Supplier
The fifth error is expecting EF-P to rescue every proline problem. EF-P abolishes stalling at polyproline stretches but has little or no effect on RxPP, DTS — stop, or Glu-Pro-stop stalling (Nascent peptides that block protein synthesis in bacteria).
Next Steps for a Sequence You Already Suspect
Start with the sequence file, not the expression run. Mark every C-terminal Pro within two residues of a stop codon, every run of three or more consecutive prolines, and the identities of positions 3 through 5 and position 7. Those are the features the evidence above ties to stalling, and they are visible before any reagent is committed.
Then decide the route. If the flagged features are present and the quantity is small to medium, chemical synthesis removes the ribosomal constraint, consistent with the pattern that 31 ar 38 recently approved small peptide drugs are chemically synthesized (Chemical vs. Recombinant: The Manufacturing Decisions Behind Blockbuster Peptide Drugs, Decibio, 2026). If the sequence is clean and the quantity is large, the construct levers, host choice, and the analytical package above are the ones to specify.
Write the specification before production. State the target purity, enfoque analítico, the requested documentation, and any special project expectations, and require lot-specific HPLC and MS data that resolve the truncated species from the target against the stated method. ICH Q6B’s requirement that identity tests be highly specific to the molecule, with more than one test where necessary, is the floor rather than the ceiling (ICH Q6B, ICH, 1999).
One limit should travel with the plan. No source read here reports a measured seconds-scale residence time for a nascent peptide in the tunnel, and the escape times from simulation, microseconds to milliseconds, have not been experimentally validated (Three epochs of nascent protein translocation through the ribosome exit tunnel, arXiv preprint). Residence time is a derived quantity, and any supplier conversation that treats it as a measured constant is ahead of the evidence.
nt'a̲ni frecuentes
Does the exit tunnel’s width limit which peptides can be expressed?
No. The tunnel is wide enough for a fully extended chain and even an α-helix, so size alone rarely blocks expression. The limit is kinetic: a sequence that holds the nascent chain in the tunnel too long, or in the wrong register, can stall elongation or interfere with release. Width sets the geometry; timing sets the outcome.
Ya pérdida ne truncamiento xkagentho nts'oki?
No, and treating them as one sends troubleshooting in the wrong direction. Stalling is a pause in elongation, and the ribosome can often resume once the obstacle clears. Truncation is the permanent result: the ribosome terminates early, or the full-length product is degraded, and the shorter chain is what you recover. A stall that resolves leaves no truncated species; a stall that does not resolve usually does.
Honja mä 'nar hñäki ngehnu̲ traducción 'nar hñäki solubilidad?
Look at where the product goes, not just how much you get. A translation-side problem gives a ladder of shorter bands on gel, which points to premature termination inside the tunnel. A solubility problem gives the right molecular weight in the insoluble fraction, with little or none in the soluble pool. Run both fractions before changing the construct, because the fix is different for each.
optimización ar codón to rescatar 'nar motivo pérdida?
Synonymous codon changes preserve the encoded peptide motif but can alter translation kinetics and mRNA behavior. They may affect expression or pausing in some contexts without necessarily removing a peptide-mediated arrest mechanism. Test the proposed change experimentally.
Temu̲ ar especificación pureza bí adapta 'nar secuencia hñei?
Set the target before production, a. A 95% Especificación to adaptar ar bí xingu flujos ar 'be̲fi nthoni ne crizado, mente 98% may be selected for demanding analytical, biológicas, or formulation-sensitive work; higher purity can improve interpretability but may raise cost and lower yield for a difficult sequence. Identity should be confirmed by tests highly specific to the molecule, with more than one test where necessary (ICH Q6B, ICH, 1999).
ar tsa̲ da utilizar ar estimación ar pa residencia predictivamente nu'bya xtä?
Not as a quantitative predictor. The residence-time figures come from structural and single-molecule work on specific sequences and conditions, and they are not a general model that takes an arbitrary sequence and returns a stall probability. Use them to reason about which constructs carry higher risk and to decide what to measure, then confirm with your own expression and characterization data.
Njäts'i nu'bu
The design response follows from those anchors. Flag C-terminal Pro adjacent to a stop codon, flag runs of three or more prolines, check positions 3 through 5 and position 7, and choose the host with the elongation rate in mind. Where the flagged features are present and the quantity is small to medium, chemical synthesis removes the ribosomal constraint; where the sequence is clean and the quantity is large, the construct levers and the analytical package carry the risk.
Two limits should travel with any decision. Residence time in the tunnel is a derived quantity, not a measured constant, and the simulation-based escape times have not been experimentally validated. The distance from the PTC to the constriction was not confirmed in the sources read here. A supplier conversation that is precise about those limits, and about the lot-level HPLC and MS data that will resolve a truncated species from the target, is the one that will hold up when the next run is compared to the last.
About the publisher. MOL Changes is a peptide research and development organisation that offers custom sequence design, synthesis and production, including solid-phase and microbial fermentation routes. It therefore has a commercial interest in how difficult sequences are made, and readers should weigh its perspective with that in mind. The guidance above stands on its own and does not depend on its services.